


Feeding Behaviours in Wild Wolves
by
Gemma Pinkard
Declaration
This dissertation is a product of my own work and is not the work of any collaboration.
I agree that this dissertation may be available for reference and photocopying at the discretion of the University and give permission for Hartpury Library Services to hold and make available an electronic copy.
Name: GEMMA PINKARD
Date: 20th March 2024
E-mail address: gemma.pinkard@hartpury.ac.uk
Faculty/ School: HARTPURY UNIVERSITY
Student name: GEMMA PINKARD
Award: BSc (Hons) CANINE TRAINING AND PERFORMANCE
Module: ANIMAL AND AGRICULTURE DISSERTATION
Project/dissertation title: FEEDING BEHAVIOURS IN WILD WOLVES (CANIS LUPUS)
Acknowledgements
Firstly, I would like to thank my dissertation supervisor, Clare Thomas-Pino for all her guidance, knowledge and support throughout my dissertation. I would also like to say a huge thank you to Tony and the wolves at wolf watch UK. They welcomed me to the sanctuary and put everything possible in place to make this study happen. Thank you to Carol Stephens for all the study skills help I received along the way. I want to say a huge thank you to my mum Jenny Pinkard for keeping me on track with continued support.
A special thank you goes out to my dogs Loki, Blade and Ghost for being my emotional support at university.
ABSTRACT
Wolves (Canis lupus) have been studied extensively for many years, however, there has been limited data collection around feeding ecology. Secretive feeding, shyness, and living in extensive landscapes, have restricted access in observing this species in proximity, and ethically has been restricted due to intrusiveness of researchers. Continuing research produces a greater understanding of wolf behaviour around feeding, and how this affects social ecology. Here we assess how wolves change actions under the influence of external and internal factors or characteristics when feeding, and whether sex is a significant influencer.
A sample of two grey wolves were used as study subjects. The wolves were siblings and included one female and one male, that live as wild in a sanctuary. The researcher was positioned in an observational hide, with the wolves unaware of the presence of the observer. Dead kills were left, and quantitative data was collected by observing each wolf feeding behaviour, and documenting on an ethogram compiled by published literature. Video cameras, a camera, and iPhone were setup, to objectively record each session, and footage was viewed to identify any other types of behaviour not recordable on the ethogram. The results demonstrate the dominance of the female wolf and the high levels of aggression that individual displays when approaching and consuming prey, compared with a male showing submission in all behavioural categories of the ethogram. The study did not reveal any findings of social pack dynamics, and the male only showed live prey hunting behaviours. Distinct feeding behaviours were identified, and the importance of understanding male and female feeding ecology, and the roles they play.
CHAPTER ONE – INTRODUCTION
1.0 Introduction
1.1 History
Wild wolves (Canis lupus) are carnivores that feed primarily on meat (Vonholdt et al. 2020). Extensive studies however have failed to clearly evaluate species feeding ecology. Dietary data is limited to published literature that is often based on one common bioregional location (Newsome et al., 2016). Published literature however supports predictions of ecological significance (Mech, 2012) and prevents miscalculations (Lindenmayer et al., 2010). Newsome et al. (2016) concluded grey wolves diet varies on location, however, findings from southern Europe indicate grey wolves switch diets from domestic species to those available (Packard, 2018).
1.2 Ecology of wolf pack dynamics
Interbreeding of Scandinavian wolves is common due to small numbers existing globally. Smeds and Ellegren (2022) however limited the study to 73 wolves over 30 years. A larger pack number would have given a preponderant data pool to a field lacking in ecological research. An ethical consideration is small sample sizes suffer repeated intrusiveness by humans over a long period of time. Habituation to humans changes natural behaviours and can cause threatening displays of behaviour in feeding to conditioned ones (Løe and Röskaft, 2004). The reliability of the research therefore is questionable. Hand fed pups are often tame, however wolves indirectly fed by humans are wild (Fritts et al., 2003). Fear of humans is a major obstacle in studies involving data collection (Mech and Janssens, 2021). Long range scopes are used, and wolves are viewed from miles away. Incorrect classifications of specific behaviours related to a specific wolf therefore are often collated, making the results unreliable. Hierarchy is established among siblings when parents leave. In a study of 19 artic wolves in Moravia, Czech-Republic, Cafazzo et al. (2016) found no substantial differences between sex. Female-male pairs were less submissive, aggressive or dominant compared with female-female, and male-male pairings. Wolves were however observed in a captive environment. Captive environments restrict inherent behaviours being performed, along with hunting behaviours of live prey (Clubb and Mason (2003); Mason, (2010).
Northern grey wolves demonstrate complex social intraspecific behaviours within packs (MacDonald et al., 2004), however each wolf makes individual decisions and weighs up the costs/benefits of fighting. Males are more aggressive than females and repel rival opponents, and females chase away pack mates (Cassidy et al., 2017). Aggression however is due to K locus genes and inherent traits (Smith, Stahler and MacNulty, 2020). Newer research needs exploring in this area. Wolves are social where pack-mates are generally related, and hunt together (Mech and Boitani, 2003). High-ranking wolves can become subordinates to their pack mates and behave more defensively and shy (Packard, 2003). However, play can lower the occurrence of aggression in established hierarchies. Dominant relationships develop in mixed aged packs, but not puppy packs (Cordoni and Palagi, 2016). There is no comprehensive contrast in play types, and future studies could help researchers appreciate the roles of play. Social play is displayed more frequently than solitary play but Cordoni (2009) used captive wolves as study subjects.
Larger body size restricts locomotor performance and restricts foraging and predator trade-offs in male wild wolves. Nevertheless, males have better handling ability of large prey. Males therefore are better attackers, selectors and killers of prey (MacNulty et al., 2009). Smaller female wolves are faster than male counterparts and demonstrate quicker bursts of acceleration and better manoeuvrability (Biewener 2003; Dial, Green and Irschick, 2008). Nilsson and Bronmark (2000) and Herrel and O’Reilly (2006) concluded however males have increased gape capacity and bite strength for successfully taking down larger prey.
1.3 Hunting
Wolves can be extremely secretive when consuming food. Observational research is difficult to conduct in the wild (Ruth et al., 2019), cumulating in a lack of research in this area. Common hunting behaviours of live prey include ambushing, relay chasing and lie in wait (Peterson and Ciucci, 2003; Mech, 2007). Relay running is a cooperative behaviour involving the continuous chase and directing of prey, and members play different roles (Peterson and Ciucci, 2003). Observational research however can be subjective and contain personal bias. Feeding consists of hunting, searching and attacking prey. Grey wolves recognise the location of prey and encircle them. The hunt is controlled by the alpha, and the beta and delta wolves come together for the attack (Mirjalili, Mirjalili and Lewis, 2014). The Grey wolf optimizer is validated by current research (Storn and Price, 1997; Askarzadeh and Rezazadeh, 2012; Gandomi and Alavi, 2012). Wolves approach prey and maintain a safe distance until contact. Once in proximity to the prey, wolves move away from each other. When the hunt is concluded wolves lay down or maintain stationary positions (Muro et al., 2011). Cordoni (2009) found wolves substantially decrease playful activity in high conflict contests, such as feeding. The study however was conducted in a captive environment and not the wild. Therefore, dead prey provided does not replicate live prey behaviours observed in the wild.
Wolves consume carrion, rich in nutrient-detritus in the form of dead animal tissue (Smith, Stahler and MacNulty, 2020). Primary food selection in wild wolves is roe deer, with less kills of smaller prey (Jędrzejewski et al., 2012). However, this is based on geographical area and prey availability. Studies on large predator-prey relations are often restricted due to the availability of the predator’s main prey (Sand, et al., 2016).
Wolves eat a diversified prey species based on prey abundance in territories.
Functional response is the relationship between kill rate and prey abundance (Smith, Stahler and MacNulty, 2020). Prey abundance on the landscape is the most important factor impacting the figure of prey killed per predator (Holling, 1959). Scandinavian wolves are flexible in changing species selection as a pack or an individual (Sand et al., 2016). Sanctuary wolves have fewer captive restrictions with home ranges in a quieter setting, and feed on live prey as consumed in a wild environment, that includes, foxes (Vulpes), magpies (Pica) and ravens (Corvus) (Wilmers et al. 2003).
Pack foraging is common in wolves that hunt large ungulates. Defending territory is essential, and the risk of food loss to scavengers is great (Mech, 1999; Fuller, Mech and Cochrane, 2003; Vucetich, Peterson and Waite, 2004). Intraspecific competition affects pack dynamics in wolf populations. Smaller packs benefit from more territorial availability (Hochard, 2014). Intraspecific clashes of aggression can result in fatalities (Mech and Boitani, 2003). Nevertheless, non-reproductive wolves are not fixed to a den and travel throughout territories together (Cassidy et al., 2015). Globally the wolf home range size relates unfavourably to prey biomass, and pack density. Pack size, scope, and human density mirror larger home ranges (Ballard, Whitman and Gardner, 1987; Wydeven, Schultz and Thiel, 1995; Okarma et al. 1998; Fuller, Mech and Cochrane, 2003; Nowak, et al., 2007; Rich et al., 2012). Results however from these studies have been inconsistent due to factors influencing social and ecological circumstances (Mattisson et al., 2013; Rich et al., 2012) prey species choice (Fuller, Mech and Cochrane, 2003), and landscape characteristics equate with hunting success (Kauffman et al., 2007; Rich et al., 2012). Each play an equal role in balancing this effect. Inconsistencies between studies furthermore demonstrate home ranges are convoluted and influenced by social and ecological factors. Detailed observations of free-ranging wolves provide a more robust insight into territoriality, territory patrol, and neighbour competitiveness (Mech and Boitani, 2003). However, the study only used a Global Positioning System (GPS) on collared wolves and was not correlated across a wider wild wolf population.
1.4 Behaviour
Hunt success is based on intra-pack familiarity, cooperation, communication and protecting group resources (MacNulty et al., 2012). However, Cassidy and McIntyre (2016) concluded inter-pack relations had a higher risk of aggressive encounters, that are most frequent in the winter months leading to breeding season. Female oestrogen and male testosterone rise to a peak in February (Asa, 1997). Grey males are more aggressive compared with females, but pack size, age and being backed by pack mates greatly influences this finding (Smith, Stahler and MacNulty 2020). Cortisol levels in greys are higher than black coated wolves (Cassidy et al., 2017). However, newer research concludes black coats are highly aggressive, and aggression is directly attributable to species-specific genes. Ethically the findings of the study by Smith, Stahler and MacNulty (2020) were based on observations with Cassidy (2017) darting wolves to take saliva swabs. The question remains, how can high cortisol levels be reliably used when wolves are darted. Cassidy and McIntyre, (2016) conducted an observed study over 5,300 days into aggression in wolves. However, only six aggressive related encounters were recorded and discussed, concluding aggression between intra-pack families is low. Escalation to an attack is contact manifested as biting (Cassidy and McIntyre, 2016). However, defining behaviour through observations during data collection can be impeded by multiple aggressive encounters occurring at once (Cordoni and Palagi, 2016). Low ranking wolves submit to dominant counterparts by lowering their posture, licking the others’ mouth, wagging the tail and lowering ears and head (Baan, 2014). Behaviours were categorised by skilled animal behavioural identification specialists, and video recorded for objectivity.
Offensive behavioural patterns of play can be defined as play ambush, play bite, play jump, play paw and play run (Cordoni, 2009). The highest rank wolf commands play demonstrating competitiveness in the species (Cordoni, 2009; Smuts, 2014). Chasing is part of play and is observed when carcass feeding (McIntyre, 2019). During the absence of parents, siblings fight for alpha and beta status (Packard, Mech and Boitani, 2003). Through play, adult wolves obtain information of both the physical and cognitive skills of others for future challenges of successive position (Cordoni, 2009; Mech and Boitani, 2003). Female wolves have established themselves as alpha status in observed packs in Yellowstone (McIntyre, 2022). Many pack decisions are decided by the Alpha female (McIntyre, 2019), who dominate other females and have killed pups to retain resources for their own litters. Alpha females will fight males interspecifically and independently (McIntyre, 2022). However, other females have used cooperation over aggression in pack leadership. Alpha females start the chase and take down live prey (McIntyre, 2019). Younger wolves display kleptoparasitism and stash food away from the kill site, before returning to the carcass to feed. Subordinates challenge for food access and social relationships affect peaceful feeding and tolerance (Range and Virányi, 2015).
Tail position is the most reliable signal of social status. The baring of teeth however is not mirrored with dominant relationships (Fatjó et al. 2007). Dale et al. (2017) used animal carcasses to assess social relationships in wolves and concluded scent marking is a non-aggressive behaviour. Defecation and urination are scent marks left for other wolves to recognise conspicuous areas, and mark territories. Females urinate and males directly urinate over the top (Smith, Stahler and MacNulty, 2020).
1.5 Ecosystem effects and species interactions
Wolves will locate dens optimally near food supplies, and Alaskan wolves select sites that clear of snow expeditiously (Joly, Sorum, and Cameron, 2018). Seasonal variation can substantially affect kill rate due to limited prey abundance specifically in winter (Sand et al., 2008; Knopff et al., 2010; Metz et al., 2012). Nevertheless, Sand et al. (2016) found snow depth in winter or other predator related factors did not affect the prey kill rate in wolves. Wolves prefer to eat in the nocturnal hours, to avoid humans and increase hunting success in the twilight hours (Eggerman et al., 2009). The study by Sand et al. (2016) did not carry out observations of kill rate during the night, concluding the data of their study is not a true representation of consumption.
1.6 Rationale
The current study is unique. There appears to be much unpublished data on wolf feeding environmental science. Therefore, further research is essential to support studies that can facilitate wolf-feeding investigations (Baumann et al., 2021). The environment in which the wolves were observed in this study are unlike anywhere else globally. Furthermore, the wolves are not viewed daily unlike in zoos that restrict natural behaviours. The wolves only see the same person each day for feeding. Therefore, the data collection of the current study is distinctive, and could contribute to a significant scientific breakthrough in supporting current research, and providing new data for analysis that future studies can be built upon.
1.7 Research aims and objectives.
The overall aim was to gather scientific data through observational research on wolf feeding behaviours between male and female wolves, recorded around pre-feeding, feeding, and after feeding has finished. A further aim was to determine common behavioural trends, other behaviours, stereotypies, or those that are less frequent over three sessions.
To address the overall research, aim the objectives were:
- to conduct three observational visits at a wolf sanctuary in England.
- to capture data of two sibling wild wolves by completing ethograms and videoing the pair of wolves during feeding times of kill provided.
- to complete behavioural analysis to identify behaviour types and trends.
CHAPTER TWO – METHODS
2.0 Methodology
Many researchers have utilised observations to measure behaviour in wolves (Fatjó et al. 2007; Cubaynes, Macnulty, Stahler 2014). Currently however study on species feeding ecology in wild wolves is extremely limited (Newsome et al., 2016). Many studies have focused on wolves in captive environments (Piffare et al., 2012; Irene et al., 2019) or have conducted studies viewing wolves from great distances questioning the validity of results. These differences employ the need for different methods of observation for assessing feeding behaviours in wild wolves.
2.1 Study Design
Between November and December 2023 three observational sessions took place at a sanctuary in Shropshire, lasting 60 to 90 minuets. The enclosure was environmentally wild, with rock faces, densely populated pine trees, wild grasslands, and a lake, that replicate wild wolf territories (Figure 1, Figure 2, Figure 3). Prior to commencing the study, the researcher conducted a site visit in November 2023. The advantage of a site visit prior to the study starting enabled the observer to understand the physical environment, talk with professionals onsite and to foresee any potential limitations or mistakes that may impact with the data collection. The site visit identified a den close to the feeding location. Therefore, the likelihood was greater of the wolves coming out to feed during the observations (Joly, Sorum and Cameron, 2018).
Nonetheless, no pilot study was conducted because of limited access to the research site. An advantage of a pilot study would have highlighted the need for a longitudinal study, in particular the analysis of feeding behaviours were restricted when wolves took the food into cover.


A signed learning agreement (See appendix A), Project proposal form (See appendix B) were completed at the start of the study. Prior to commencing the study, ethical clearance was sought from Hartpury Ethics committee (ETHICS2023-88-LR) (See appendix C) and was granted. A site permission form (See appendix D), a risk assessment (See appendix E) and Hazard risk assessment completed prior to starting the study (See appendix F).
Observational field studies are a key method to collect information gathered by experimental methods to characterise ecological legitimacy (Komulainen, 2022). The present study uses an ethnographic approach including an ethogram (See appendix G, H and I) to measure the behavioural responses of wolves when feeding. The ethogram was completed manually at the time the behaviour was observed. The ethogram was selected for quantitative reliability and validity and was based on the one adopted by The International Wolf Sanctuary. Quantitative variables are known as continuous and quantitative research gathers data analysed through numbers (Hawkins, 2019, p.255). Ethograms have previously been chosen to give a detailed understanding of classifying large carnivore behaviours (Goodmann et al., 2002; Frézard and Pape, 2003; Mech and Boitani, 2003; Pifarré et al., 2012). In observational studies there is potential bias from observers. To rule out this possibility, all sessions were recorded using a Sony camera and Apple Iphone. The wolves were observed from a close vantage point (See figure 4). The design of the lookout is rustic and blends in with the environment. The lookout is elevated, and positioning stops the observer being scented or seen. Natural behaviours can then be displayed around the kill. A major advantage was the observer being able to clearly identify the behaviour being displayed, and by what wolf. Previous research has relied on scopes viewing wolves from great distances, often resulting in incorrect identification of individual behaviours, or being unable to record multiple behaviours from multiple wolves occurring at once (Janssessens and Mech, 2021).

On arrival at the sanctuary the time to bring the kill to the feeding site was agreed upon by the observer and the sanctuary owner. To rule out the possibility of influence of behaviour, the same daily feeding site was used. The location is the brown feeding spot (figure 5).

The observer entered the hide and set up the cameras The wolves came into the open when the food was brought to the site. Data was collected when the wolves started to interact in anyway with the feeding process. It was not possible to investigate the significant relationships of feeding behaviours in sessions one and two extensively due to the time the wolves spent feeding in cover. A causal factor could be the weather conditions of strong wind and heavy rain. Wolves save energy by not hunting in wind and rain. Further data collection is required to determine exactly how the weather affects feeding behaviour. The observations were not finished until the wolves had consumed all the food and had gone back into cover.
2.2 Sampling
The sample size was a wild pack of two nine-year-old sibling Norwegian Grey Wolves. Rickon, a male, and Sansa a female. A small sample size is justifiable for furthering essential research into feeding ecology in wild wolves.
Wolf one: Identifiable as smaller than brother Rickon, Sansa has black along the spine, that clusters in a square mid back, and on the tip of the tail (Figure 6).

Wolf two: As a male Rickon is structurally bigger than Sansa. Rickon has a darker pigment on the face, but whiter block colour on the torso (Figure 6).

2.3 Data analysis
The raw data from the three ethograms (See appendix G, H and I) was collected and input into an Excel spreadsheet (See appendix J). Pie charts were generated for each of the sessions to illustrate the individual behaviours of each wolf exhibited (Field, 2017). In addition, a bar chart was created to visually represent the frequency of individual behaviours (Hawkins, 2019). Subsequently, thematic analysis was conducted to identify key trends and patterns, which emerged from the raw data and descriptive statistics (Braun and Clarke, 2006). The camera footage captured was viewed and analysed in its entirety. The analysis entailed looking for any other types of specific behaviour not documented on the ethograms. This was justified to generate further added evidence of behaviour not documented in the ethograms.
A positivist approach was adopted which is appropriate for quantitative research methods (Cottrell, 2014). A positivist research philosophy takes the view only factual knowledge through observation, including measurement, is reliable. Positivism addressed the research aims in this study (Clark et al., 2021). Data collected is a natural study as data was collected in the field. Scale (counts and measures) allows the difference between values to be measured. The scale method is a strongest level of measurement compared with nominal (categories) measurement (Hawkins, 2019)
2.4 Ethics
No data was collected before ethical clearance was granted by the Hartpury Ethics Committee. For ethical reasons the decision was made that the wolves were only exposed to one experimental condition. Moreover, with the researcher observing from the hide, there was no direct contact with the wolves, and the researcher could not be seen. Therefore, the research was not intrusive and in no way could cause any physical or psychological harm (Cottrell, 2014). Anonymity and confidentiality were maintained (Whisker, 2019). The data was stored securely on the Hartpury One Drive, and password protected, in accordance with the General Data Protection Regulations (GDPR), and the Data Protection Act 2018 (GOV.UK). Researcher bias was avoided as far as possible through the quantitative ethogram data collection method supported by the objective video evidence.
CHAPTER THREE – RESULTS
3.0 Results
3.1 Ethogram results
The data from the three ethograms (See appendix G, H, and I) were analysed and identified nineteen key behaviours, and ‘other’ behaviours around feeding in wolves.
Table 1: showing the summary statistics for frequency and the mean of feeding behaviour, recorded over the three sessions.
| Behaviour | Session 1 | Session 2 | Session 3 | Mean (Average) |
|---|---|---|---|---|
| Relay chasing | 5 | 1 | 3 | 3 |
| Circling prey | 3 | 1 | 3 | 2 |
| Hunting live prey | 0 | 1 | 8 | 3 |
| Stalking/Hurding | 2 | 1 | 2 | 2 |
| Tall position changes | 4 | 1 | 7 | 4 |
| Aggression | 4 | 4 | 38 | 15 |
| Escape | 1 | 1 | 4 | 2 |
| Indirect approach | 2 | 1 | 4 | 2 |
| Centuary/territory checking | 5 | 3 | 1 | 3 |
| Follow | 3 | 1 | 5 | 3 |
| Vocalisations | 0 | 1 | 0 | 0 |
| Body posture changes | 2 | 1 | 9 | 4 |
| Urination/defication | 1 | 0 | 5 | 2 |
| Changes in play | 0 | 0 | 0 | 0 |
| Approach | 0 | 1 | 8 | 3 |
| Creep/crawl/crouch | 0 | 0 | 5 | 2 |
| Submissive behaviour | 3 | 1 | 7 | 4 |
| Critical reaction | 0 | 0 | 3 | 1 |
| Leave | 0 | 1 | 0 | 1 |
| Other behaviours | 0 | 1 | 8 | 3 |
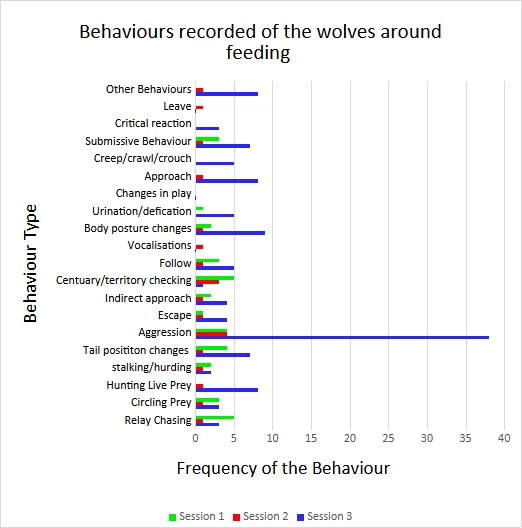


Table 2: The breakdown of results obtained of pack hierarchy and feeding behaviour in sessions 1-3. Analysis of the data was compared between male and female sex.
| Behaviour | Female | Male | Female | Male | Female | Male |
|---|---|---|---|---|---|---|
| Session number | 1 | 1 | 2 | 2 | 3 | 3 |
| Searching for live prey | No | No | No | Yes | No | Yes |
| Ambushing live prey | No | No | No | No | No | Yes |
| Relay chasing live prey | No | No | No | No | No | Yes |
| Circling Live Prey | No | No | No | No | No | Yes |
| Working as an equal pack | No | No | No | No | No | No |
| Maintaining distance from prey | No | Yes | Yes | Yes | No | No |
| Circling when prey brought to site | No | Yes | Yes | Yes | Yes | Yes |
| Approaching food as an equal pack | No | No | No | No | No | No |
| Confident in approaching food from human | No | No | Yes | Yes | No | No |
| Eating first | Yes | No | Yes | Yes | Yes | No |
| Consumed the most food | Yes | No | Yes | No | Yes | No |
| Aggressive around feeding | Yes | No | Yes | No | Yes | No |
| Eating in cover | Yes | Yes | Yes | Yes | No | No |
| Eating in the open | No | No | No | No | Yes | Yes |
| Decrease in play | Yes | Yes | Yes | Yes | Yes | Yes |
| Urinate during feeding | Yes | Yes | Yes | Yes | Yes | Yes |
| Defecate during feeding | Yes | Yes | Yes | Yes | Yes | Yes |
| Leader in the follow | Yes | No | Yes | No | Yes | No |
| Leader in relay chasing | Yes | No | Yes | No | Yes | No |
| Dominant wolf | Yes | No | Yes | No | Yes | No |
| Submissive wolf | No | Yes | No | Yes | No | Yes |
| Other behaviour | No | No | No | No | Yes | No |
Notes were made on the ethogram (See appendix G, H and I) for behaviours not listed, these are recorded as ‘other’ behaviours. Observed behaviours classed as ‘other’ included scent marking and returning to a den close to the feeding site in session 3. Both behaviours were performed by the female wolf. Session 3 also observed the female stashing food and aggressively defending it.
3.2 Video results
Video recorded sessions were watched in full and any ‘other’ behaviour displayed were recorded manually on the ethogram to ensure no duplication of results.
CHAPTER FOUR – DISCUSSION
4.0 Discussion
4.1 Introduction
There is global interest in feeding ecology in wild wolves. However, secretive feeding (Ruth et al., 2019) and large territories hinder the success of gathering scientific research through observational studies. This has directly resulted in a significant lack of rich and up to date data in feeding behaviours. This study aimed to provide scientifically reliable data directly related to behaviours exhibited by both male and female wolves, during the feeding process.
4.2 Pack hierarchies
The current investigation found no evidence of social pack dynamics. What is striking in table 2 is that across all 3 sessions the wolves did not work as an equal pack when food was brought to the site, or approach food as an equal pack when it was left. The discrepancy could be attributed to food being provided daily so there is little need to hunt. The study was unable to demonstrate that wolves are social and hunt together when pack mates are related in contrast to earlier findings of Mech and Boitani (2003). An interesting finding was the male wolf did not at any time challenge the female for alpha status and remained the subordinate wolf. This inconsistency maybe due to only a small sample size of two wolves being used. Packard (2003) showed that high-ranking wolves can become subordinates to their pack mates and behave in a shy manner, and that in the absence of parents, siblings fight for alpha and beta status. This differs from findings presented here. The study established the male demonstrated submissive behaviour across all three sessions to the female who remained the alpha wolf, and as siblings they did not challenge for pack status. What is interesting, is figure 9 has the highest frequency of submissive behaviours at 9% in session 1, but session one had the lowest aggression score at 11%. An alternative explanation for the result is that it was due to the wolves only being observed for a short time before they returned to cover. This study is consistent with Bann (2014) who concluded lower ranking wolves will submit to higher ranking wolves. Further research is needed to explore the mechanisms between siblings in packs.
4.3 Aggression
The results in this study found female grey wolves are more aggressive than male counterparts when consuming food. Figure 8 indicates there was a sharp increase in the number of recorded aggressive encounters in session 3. The possible explanation might be the wolves spent more time in the open so were observed for longer. However, an alternative explanation for this result is that this is a true reflection of what intraspecific aggressive behaviours around feeding occur naturally in the wild. The outcome of this result is contrary to the findings of Cassidy et al. (2017) who reported males being more aggressive than females. Another finding is the female chased away the male four times in session 3, and strikingly table 2 shows the male did not display any signs of aggression to the female across all three sessions. This intriguing result might have been attributed to the female being of alpha status in the pack. However, these results support previous observations of Cassidy et al. (2017) that females chase away pack mates, and males only fend off rival opponents, which could be a causal factor in the result. On the question of aggression this study found aggressive behaviours in all three sessions. What clearly stands out in figures 9, 10 and 11 is aggression has the highest percentage of observed behaviours. Several factors could explain this result. Firstly, aggressive encounters are highest in the winter months, when female oestrogen and male testosterone levels rise to peak in February as reported by Asa (1997) and Smith, Stahler and MacNulty (2022), who also conducted observations during the winter months. The most obvious findings to emerge from the analysis of aggressive encounters is that the lunge along with the approach were the most frequently displayed behaviours across all three sessions. This finding can be attributed to food becoming available/left at the kill site, and the consuming of food at this time. What stands out in table 2 is the female wolf eats first, consumes the most food, and was dominant in all three sessions. Table 1 clearly shows 9 incidents of body posture changes in session 3, and figure 12 shows a gradual increase of aggressive behaviours being observed across all 3 sessions. What clearly stands out in figure 12 are highly aggressive behaviours of ritualised attack, give eye and baring of teeth evident in session 3. The outcome is contrary to that of MacNulty (2012) who concluded that aggression between intra-pack families is low. No aggression was displayed when all food was consumed.
4.4 Hunting
As mentioned in the literature review common hunting behaviours of live prey include ambushing and lie in wait (Ciucci, 2003; Mech, 2007). The study further supports this idea as ambushing is seen, but in figure 2 relay chasing and searching for live prey were demonstrated. One unanticipated result was the male only displayed hunting live prey behaviours. However, the inconsistency may be due to the wolves relying on food being provided, and that the female ate most food in the sessions. The live prey species in session 3 was a magpie which supports the findings of Smith, Stahler and MacNulty (2020) and Wilmers et al. (2003), who found captive wolves feed on magpies as they would in the wild. In this study when food was brought close to the kill spot the wolves did not move away from each other. This outcome is contrary to that of Munro et al. (2011) and Cordoni (2009) who found that wolves move towards each other. The results of this study did however reflect those of Munro et al. (2011) and Cordoni (2009) observations of wolves decreasing playful activity during feeding, and maintaining stationary positions once feeding was concluded. However, these data must be interpreted with caution because food was provided by a human, and not replicable of prey consumed in the wild.
4.5 Other behaviours
When food was left, the male was observed in video analysis slinking behind the female and backing off to allow her to eat first. This supports McIntyre (2022) that females have established themselves as alphas in established packs, and pack members play different roles (Peterson and Ciucci, 2003) but is contrary to findings by Caffazzo et al. (2016) who found no substantial difference between sex.
Another important finding is changes in tail positions across all three sessions. Each ethogram (see appendix G, H, and I) significantly found that tail position 4 (tail between legs) was the only position demonstrated by the male in all feeding sessions. This finding broadly supports the work of Fatjó et al. (2007), who linked tail position changes as the most reliable signal of social status. It is possible the results in this study may underestimate the role of tail position in each session due to the partial consuming of food in cover in sessions 1 and 2, so feeding behaviour could not be fully observed.
Perhaps the most interesting finding in session 3 was the display of kleptoparasitism and stashing of food away from the kill site by the female, who aggressively defended the food from the male. This finding of stashing food by younger wolves and challenging by subordinates was reported by Range and Viranyi (2015). In contrast, however, the study did not provide evidence of male wolves stashing the food as reported by McIntyre (2019). A note of caution is due here since a sample of only two wolves was used, and the wolves were only observed consuming all food in the open in session 3. This behaviour may not have occurred in consumption of food in cover in session 1 and 2. Therefore, further investigations are needed to confirm or validate these findings.
Nothing was found in the literature review of females rubbing their necks into the ground after feeding. However, this study observed this behaviour. These findings may be taken to indicate scent marking, but it is possible that these results do not represent this behaviour. Further investigations are required to determine whether this behaviour is linked to scenting. What can clearly be seen in figure 9 and 11 is the frequency of defecation and urination in these sessions, and table 2 clearly shows both sexes performed this behaviour during feeding. However, the findings of the current study do not support previous research by McIntyre (2019) that defecation and urination are scent marks left for other wolves, and that when females urinate males will urinate directly over the top. Therefore, these findings are disappointing. To develop a full picture of urination and defecation in feeding additional studies will be needed to establish how this behaviour is linked to feeding. In summary, the results of this observational study indicate female wolves exhibit alpha status behaviours in the feeding process and show high levels of aggression to subordinate wolves when consuming food.
4.6 Study limitations
A limitation of this study is the small sample size, which means the findings cannot be generalised to a wider population (Wisker, 2019). A further limitation was not all the behaviour could be observed or filmed due to the wolves eating in cover. Observational studies can be more prone to subjectivity however, this was mitigated using video data capture and a scientifically evidenced-based ethogram.
4.7 Future research
Further research using a longitudinal observational study would establish larger data collection and allow for the development of more specific and reliable analytical method for statistical analysis. Previous research has been extremely limited due to large distances for observing wild wolves. Further investigations into sibling behaviour would evaluate the impact of relationships on behaviour. The study however is unique and allows for accurate and valid data though close and controlled observation justifying a small sample size. Researchers can use the data collected in this study for future to research into feeding ecology in wolves.
The research generated a large quantity of raw data in the form of contemporaneous notes from the researcher. The data could have facilitated further comparisons or trends in feeding behaviours of ecological significance. The data was not used due to concerns over the validity of scoring the same behaviour twice, but future studies can draw on these findings to construct new hypothesis around feeding behaviours in wolves.
CHAPTER FIVE – CONCLUSION
5.0 Conclusion
The aim of this study was to explore the influence of feeding on behaviours exhibited by wild wolves. The research has identified distinct behaviour differences in both female and male wolves. One of the more significant findings clearly highlighted a female demonstrating dominant alpha behaviours especially when consuming the food, with a male beta wolf always being submissive to their counterpart. This study concluded subordinates will submit to higher ranking wolves. The results of this investigation report the wolves did not work as a pack when food was brought to the site, or on approaching the food when it was left. The wolves did not hunt together or demonstrate high levels of sociability as concluded in previous studies. However, relying on food being brought each day could be a contributory factor for the lack of sociability and the hunting of live prey. The study contributes to our understanding of the effects of prey abundance and the need for wolves to hunt. Another key finding was the inordinate nature of aggressive behaviours exhibited frequently throughout the observation periods, and the significance of these in both sex and the sibling relationship. Notwithstanding the relatively limited sample, this study offers some insight into how sex and sibling relationships affect pack hierarchy, sociability, and behaviour around feeding. This study lays the groundwork for future research that could beneficially explore the effects of sibling relationships on feeding using a bigger sample size. Prior to this study it was difficult to make predictions about how wolves behave around feeding. This is due to limitations of observing wolves at great distances over extensive landscapes. Nonetheless, this study is the first of substantial duration which examines associations between behaviour and feeding in wolves.
Author: Gemma Pinkard
EXPLORATORY STUDY OF FEEDING BEHAVIOURS IN WILD WOLVES (CANIS LUPUS). 20th March 2024
REFERENCES
Asa, C.S. (1997) Hormonal and experimental factors in the expression of social and parental behaviour in Canids, In cooperative breeding in mammals, edited by N.G. Solomon and J.A. French, p129-149. Cambridge, Cambridge University press.
Askarzadeh, A. and Rezazadeh, A. (2012) ‘Parameter identification for solar cell models using harmony search-based algorithms’, Solar Energy, 86 (11), pp.3241-3249.
Baan, C., et al. (2014) ‘Conflict management in free-ranging wolves, Canis lupus’, Animal Behaviour (90), pp. 327–334, Available https://doi.org/10.1016/j.anbehav.2014.01.033.
Ballard WB, Whitman JS, Gardner CL. (1987) ‘Ecology of an exploited wolf population in south-central Alaska’, Wildlife Monographs (98) pp. 5-54
Biewener, A.A. (2003) Animal Locomotion. Oxford University Press, Oxford, UK
Braun, V. and Clarke, V. (2006.) ‘Using thematic analysis in psychology’ Qualitative research in psychology, 3 (2), pp.77-101.
Baumann, C., Pfrengle, S., Münzel, S.C., Molak, M., Feuerborn, T.R., Breidenstein, A., Reiter, E., Albrecht, G., Kind, C.J., Verjux, C. and Leduc, C. (2021) ‘A refined proposal for the origin of dogs: the case study of Gnirshöhle, a Magdalenian cave site’. Scientific Reports, 11(1), pp.1-14.
Cafazzo, S., Lazzaroni, M. and Marshall-Pescini, S. (2016) ‘Dominance relationships in a family pack of captive arctic wolves (Canis lupus arctos)’, The influence of competition for food, age and sex’, PeerJ, (4) pp. 2707. Doi: https://doi.org/10.7717/peerj.2707
Cassidy, K.A., MacNulty, D.R., Stahler, D.R., Smith, D.W. and Mech, L.D. (2015) Group composition effects on aggressive interpack interactions of gray wolves in Yellowstone National Park. Behavioral Ecology, 26 (5), pp.1352-1360.
Cassidy, K.A., Mech, L.D., MacNulty, D.R., Stahler, D.R. and Smith, D.W., 2017. ‘Sexually dimorphic aggression indicates male gray wolves specialize in pack defense against conspecific groups’, Behavioural processes, 136, pp, 64-72.
Cassidy, K.A. and McIntyre, R.T. (2016) ‘Do gray wolves (Canis lupus) support pack mates during aggressive inter-pack interactions?’ Animal Cognition, (19), pp. 939-947
Clark, T., Foster, L., Sloan, L. and Bryman, A. (2021) Bryman’s social research methods. Oxford: Oxford University Press.
Clubb, R. and Mason, G. (2003) ‘Captivity effects on wide-ranging carnivores’, Nature, 425 (6957), pp.473-474.
Cafazzo, S. et al. (2018) ‘In wolves, play behaviour reflects the partners’ affiliative and dominance relationship’, Animal Behaviour, (141), pp. 137–150. doi:10.1016/j.anbehav.2018.04.017.
Cottrell, S. (2014) Dissertations and project reports: a step by step guide. Basingstoke: Palgrave Macmillan.
Cordoni, G. (2009) ‘Social play in captive wolves (Canis lupus): not only an immature affair’, Behaviour, 146 (10), pp. 1363–1385. doi:10.1163/156853909×427722.
Cordoni, G., Palagi, E. (2016) ‘Aggression and hierarchical steepness inhibit social play in adult wolves’, Behaviour 153 (6–7), 749–766.
Cubaynes, S., MacNulty, D.R., Stahler, D.R., Quimby, K.A., Smith, D.W. and Coulson, T. (2014) ‘Density‐dependent intraspecific aggression regulates survival in northern Yellowstone wolves (Canis lupus)’, Journal of Animal Ecology, 83 (6), pp.1344-1356.
Data Protection Act 2018. Available at: https://www.gov.uk/data-protection. (Accessed 4 February 2024).
Dale, R. (2017) ‘The influence of social relationship on food tolerance in wolves and dogs’, Behavioral Ecology and Sociobiology, 71(7). doi:10.1007/s00265-017-2339-8.
Dial, K.P., Greene, E. and Irschick, D.J. (2008) ‘Allometry of behavior’ Trends in ecology & evolution, 23 (7), pp.394-401.
Eggermann, J., Gula, R., Pirga, B., Theuerkauf, J., Tsunoda, H., Brzezowska, B., Rouys, S. and Radler, S. (2009) ‘Daily and seasonal variation in wolf activity in the Bieszczady Mountains, SE Poland’, Mammalian Biology, 74, pp.159-163.
Fatjó, J., Feddersen-Petersen, D., de la Torre, J.L.R., Amat, M., Mets, M., Braus, B. and Manteca, X. (2007), ‘Ambivalent signals during agonistic interactions in a captive wolf pack’, Applied animal behaviour science, 105 (4), pp.274-283.
Field, 2017 book paperback, 5th edition, sage publications
Frézard, A. and Pape, G.L. (2003) ‘Contribution to the welfare of captive wolves (Canis lupus lupus)’, A behavioral comparison of six wolf packs. Zoo Biology: Published in affiliation with the American Zoo and Aquarium Association, 22 (1), pp.33-44.
Fritts, S.H., Stephenson, R.O., Hayes, R.D. and Boitani, L. (2003) Wolves and humans.
Fuller, T.K., Mech, L.D. and Cochrane, J.F. (2003) ‘Wolf population dynamics’.
Gandomi, A.H. and Alavi, A.H. (2012) ‘Krill herd: a new bio-inspired optimization algorithm’, Communications in nonlinear science and numerical simulation, 17 (12), pp.4831-4845.
Gilby, I.C. (2006) ‘Meat sharing among the Gombe chimpanzees: harassment and reciprocal exchange’, Animal Behaviour, 71(4), pp.953-963.
Goodman, J.I. and Watson, R.E. (2002) ‘Altered DNA methylation: a secondary mechanism involved in carcinogenesis’, Annual review of pharmacology and toxicology, 42( 1), pp.501-525.
Hawkins, (2019) Biomeasurement, a guide to biological statistics. 4 edition, oxford.
Herrel, A. and O’Reilly, J.C. (2006) ‘Ontogenetic scaling of bite force in lizards and turtles’, Physiological and Biochemical Zoology, (79), pp.31-42.
Bottom of Form
Hochard, J. and Finnoff, D. (2014) ‘Grey wolf population projection with intraspecific competition’, Natural resource modelling, 27 (3), pp. 360–375. doi:10.1111/nrm.12038.
Holling, C.S. (1959) ‘The components of predation as revealed by a study of small-mammal predation of the European Pine Sawfly1’, The canadian entomologist, 91 (5), pp.293-320.
Irene, R., Barbara, R., Vallisneri, M. and Caterina, S. (2019) ‘Behavioural diversity in a zoo pack of wolves, Investigating welfare through observational variety index, pp. 1-1
Jędrzejewski, W. et al. (2012) ‘Prey choice and diet of wolves related to ungulate communities and wolf subpopulations in Poland,” Journal of Mammalogy, 93(6), pp. 1480–1492. doi:10.1644/10-mamm-a-132.1.
Joly, K., Sorum, M. S., Cameron, M. D. (2018) ‘Denning Ecology of Wolves in East-Central Alaska’, 1993 – 2017. Arctic, vol. 71(4), p 444–455. https://www.jstor.org/stable/26567073
Kardos, M., Akesson, M., Fountain, T., Flagstad, O., Liberg, O., Olason, P., Sand, H., Wabakken, P., Wikenros, C., & Ellegren, H. (2018) ‘Genomic consequences of intensive inbreeding in an isolated wolf population’, Nature Ecology & Evolution, 2(1), pp. 24–131. https://doi.org/10.1038/s4155 9-017-0375-4
Kauffman, M.J., Varley, N., Smith, D.W., Stahler, D.R., MacNulty, D.R. and Boyce, M.S. (2007) ‘Landscape heterogeneity shapes predation in a newly restored predator–prey system’, Ecology letters, 10 (8), pp.690-700.
Knopff, K.H., Knopff, A.A., Kortello, A. and Boyce, M.S. (2010) ‘Cougar kill rate and prey composition in a multiprey system’, The Journal of Wildlife Management, 74 (7), pp.1435-1447.
Komulainen, S. (2022) ‘Howl I get to know you?: a review of behavioural observation methods: implications for monitoring wild wolves’, (Bachelor’s thesis, S. Komulainen).
Lindenmayer, D.B., Likens, G.E., Krebs, C.J. and Hobbs, R. (2010) ‘Improved probability of detection of ecological “surprises’, Proceedings of the National Academy of Sciences, (51), pp.21957-21962.
Løe J, Röskaft E. (2004) ‘Large carnivores and human safety, a review’, AMBIO (33) pp. 283–288
Macdonald, D.W., Creel, S. and Mills, M.G. (2004) ‘Canid society’, The biology and conservation of wild canids, pp.85-106.
MacNulty, D.R, Mech, L.D., Smith, D.W. (2007) ‘Aproposed ethogram of large-carnivore predatory behaviour, exemplified by the wolf’, Journal of Mammalogy, (870), pp. 80-84.
MacNulty, D. R., Smith, D. W., Mech, L. D., & Eberly, L. E. (2009) ‘Body Size and Predatory Performance in Wolves: Is Bigger Better?’, Journal of Animal Ecology, 78 (3), pp. 532–539. http://www.jstor.org/stable/27696397
MacNulty, D.R, Douglas W. Smith, L. David Mech, John A. Vucetich, Craig Packer. (2012) ‘Nonlinear effects of group size on the success of wolves hunting elk’, Behavioral Ecology, Volume 23, Issue 1, pp. 75 82, https://doi.org/10.1093/beheco/arr159
Mason, G.J. (2010) ‘Species differences in responses to captivity: stress, welfare and the comparative method’, Trends in ecology & evolution, 25(12), pp.713-721.
Mattisson, J. et al. (2013) ‘Home range size variation in a recovering wolf population: evaluating the effect of environmental, demographic, and social factors’, Oecologia, 173 (3), pp. 813–825. doi:10.1007/s00442-013-2668-x.
McIntyre, R. (2019) The Rise of Wolf 8: Witnessing the Triumph of Yellowstone’s Underdog, (Vol. 1). Greystone Books Ltd.
McIntyre R. (2022) The Alpha female wolf: The fierce legacy of Yellowstones 06, Grey stone books Ltd.
Mech, L.D. (1999) ‘Alpha status, dominance, and division of labor in wolf packs’, Canadian journal of zoology, 77 (8), pp.1196-1203.
Mech L.D., Boitani L. (Eds.), Wolves: Behavior, Ecology and Conservation, University of Chicago Press, Chicago (2003), pp. 161-191
Mech, L.D. (2007) ‘ Possible use of foresight, understanding, and planning by wolves hunting muskoxen’, Arctic, pp.145-149
Mech, L.D. (2012) ‘Is science in danger of sanctifying the wolf?’, Biological Conservation, 150 (1), pp.143-149.
Mech, L.D. and Boitani, L. eds. (2019) Wolves: behavior, ecology, and conservation’, University of Chicago Press.
Mech, L.D. and Janssens, L.A. (2021) ‘An assessment of current wolf Canis lupus domestication hypotheses based on wolf ecology and behaviour.’, Mammal Review, 52 (2), pp.304-314.
Metz, M.C., Vucetich, J.A., Smith, D.W., Stahler, D.R. and Peterson, R.O. (2011) ‘Effect of sociality and season on gray wolf (Canis lupus) foraging behavior: implications for estimating summer kill rate’, PloS one, 6 (3), p.e17332.
Metz, M.C., Smith, D.W., Vucetich, J.A., Stahler, D.R. and Peterson, R.O. (2012) ‘Seasonal patterns of predation for gray wolves in the multi‐prey system of Yellowstone National Park’, Journal of Animal Ecology, 81(3), pp.553-563.
Mirjalili, S., Mirjalili, S.M. and Lewis, A. (2014) Grey Wolf Optimizer’, Advances in Engineering Software, 69, pp. 46–61. doi:10.1016/j.advengsoft.2013.12.007.
Muro, C., Escobedo, R., Spector, L., Coppinger, R.P (2011) ‘Wolf-pack (Canis lupus) hunting strategies emerge from simple rules in computational simulations’, Author links open overlay panel’, Behavioural Processes.
Newsome, T.M., Boitani, L., Chapron, G., Ciucci, P., Dickman, C.R., Dellinger, J.A., López‐Bao, J.V., Peterson, R.O., Shores, C.R., Wirsing, A.J. and Ripple, W.J. (2016) ‘ Food habits of the world’s grey wolves’,Mammal Review, 46(4), pp.255-269 doi:10.1111/mam.12067.
Nilsson, P.A. and Bronmark, C, (2000) ‘Prey vulnerability to a gap-sized limited predator; behavioural and morphological impacts on northern pike piscivory’, Oikos, (88), pp.539-546.
Nowak, S., Jędrzejewski, W., Schmidt, K., Theuerkauf, J., Mysłajek, R.W. and Jędrzejewska, B. (2007) ‘Howling activity of free-ranging wolves (Canis lupus) in the Białowieża Primeval Forest and the Western Beskidy Mountains (Poland).’,Journal of Ethology, (25), pp.231-237.
Okarma, H., Jędrzejewski, W., Schmidt, K., Śnieżko, S., Bunevich, A.N. and Jędrzejewska, B. (1998) ‘Home ranges of wolves in Białowieża Primeval Forest, Poland, compared with other Eurasian populations’, Journal of mammalogy, 79 (3), pp.842-852.
Packard, J.M., Mech, L.D. and Boitani, L. (2003) Wolves: behavior, ecology, and conservation. The university of Chicago press, Chicago. pp: 35-65
Packard, J.M. (2010) Wolf Behavior: Reproductive, Social, and Intelligent. In Wolves, University of Chicago Press, pp. 35-65
Packard, J.M., 2018. 90078 Wolves.
Peterson, R.O. and Ciucci, P. (2003) ‘The wolf as a carnivore’, In Wolves: behavior, ecology and conservation, University of Chicago Press.
Pifarré, M., Valdez, R., González-Rebeles, C., Vázquez, C., Romano, M. and Galindo, F. (2012) T’he effect of zoo visitors on the behaviour and faecal cortisol of the Mexican wolf (Canis lupus baileyi)’, Applied Animal Behaviour Science, 136 (1), pp.57-62.
Range, F. and Virányi, Z. (2015) ‘Tracking the evolutionary origins of dog-human cooperation: the “Canine Cooperation Hypothesis’, Frontiers in Psychology, (5), p.1582.
Rich, L.N., Mitchell, M.S., Gude, J.A. and Sime, C.A. (2012) ‘Anthropogenic mortality, intraspecific competition, and prey availability influence territory sizes of wolves in Montana’, Journal of Mammalogy, 93(3), pp.722-731.
Ruth, Toni K., Polly C. Buotte, and Maurice G. Hornocker, (2019) Yellowstone cougars: ecology before and during wolf restoration. University Press of Colorado,
Sand, H., Wabakken, P., Zimmermann, B., Johansson, Ö., Pedersen, H.C. and Liberg, O. (2008) ‘Summer kill rates and predation pattern in a wolf–moose system: can we rely on winter estimates?’, Oecologia, 156, pp.53-64.
Sand, H. (2016) ‘Prey Selection of Scandinavian Wolves: Single Large or Several Small?’, PLOS ONE. Edited by M. Apollonio, 11(12), p. e0168062. doi:10.1371/journal.pone.0168062.
Smeds, L. and Ellegren, H. (2022) ‘From high masked to high realized genetic load in inbred Scandinavian wolves’, Molecular Ecology, 32(7), pp. 1567–1580. doi:10.1111/mec.16802.
Smith, D., Stahler, D., and MacNulty, R. (2020) Yellow stone wolves, The University of Chicargo Press.
Smith, D.W., Drummer, T.D., Murphy, K.M., Guernsey, D.S. and Evans, S.B. (2004) ‘Winter prey selection and estimation of wolf kill rates in Yellowstone National Park’, 1995–2000, The Journal of Wildlife Management, 68 (1), pp.153-166.
Smith, D.W. (2015) ‘Infanticide in wolves: seasonality of mortalities and attacks at dens support evolution of territoriality’, Journal of Mammalogy, 96(6), pp. 1174–1183. doi:10.1093/jmammal/gyv125.
Stahler, D.R., Smith, D.W. and Guernsey, D.S. (2006) ‘Foraging and feeding ecology of the gray wolf (Canis lupus) lessons from Yellowstone National Park, Wyoming, USA’, The Journal of nutrition, 136(7), pp.1923S-1926S.
Stevens, J.R. and Gilby, I.C. (2004) ‘A conceptual framework for nonkin food sharing: timing and currency of benefits’, Animal Behaviour, 67(4), pp.603-614.
Storn, R. and Price, K. (1997) ‘Differential evolution–A fast and efficient heuristic for global optimization over continuous spaces’, Journal of Global Optimization, 11, pp.341-359.
vonHoldt, B.M., DeCandia, A.L., Heppenheimer, E., Janowitz‐Koch, I., Shi, R., Zhou, H., German, C.A., Brzeski, K.E., Cassidy, K.A., Stahler, D.R. and Sinsheimer, J.S. (2020) ‘Heritability of interpack aggression in a wild pedigreed population of North American grey wolves’, Molecular ecology, 29 (10), pp.1764-1775.
Vucetich J.A., Peterson R.O., Waite T.A. (2004) ‘Raven scavenging favours group foraging in wolves’, Anim. Behav., 67, pp. 1117-1126
Vucetich, J.A. and Peterson, R.O. (2004) ‘The influence of prey consumption and demographic stochasticity on population growth rate of Isle Royale wolves Canis lupus’, Oikos, 107(2), pp.309-320.
Wilmers, C.C., Stahler, D.R., Crabtree, R.L., Smith, D.W. and Getz, W.M. (2003) ‘Resource dispersion and consumer dominance: scavenging at wolf‐and hunter‐killed carcasses in Greater Yellowstone, USA’, Ecology Letters, 6 (11), pp.996-1003.
Wilmers, C.C., Crabtree, R.L., Smith, D.W., Murphy, K.M. and Getz, W.M. (2003) ‘Trophic facilitation by introduced top predators: grey wolf subsidies to scavengers in Yellowstone National Park’ Journal of Animal Ecology, 72 (6), pp.909-916.
Wisker, G. (2019) The dissertation research handbook. London: Red Globe Press
Wydeven, A.P., Schultz, R.N. and Thiel, R.P. (1995) ‘Monitoring of a recovering gray wolf population in Wisconsin, 1979–1991’, Ecology and Conservation of Wolves in a Changing World. Canadian Circumpolar Institute, Edmonton, Alberta, pp.147-156.
www.International wolf center (Wolf.org)